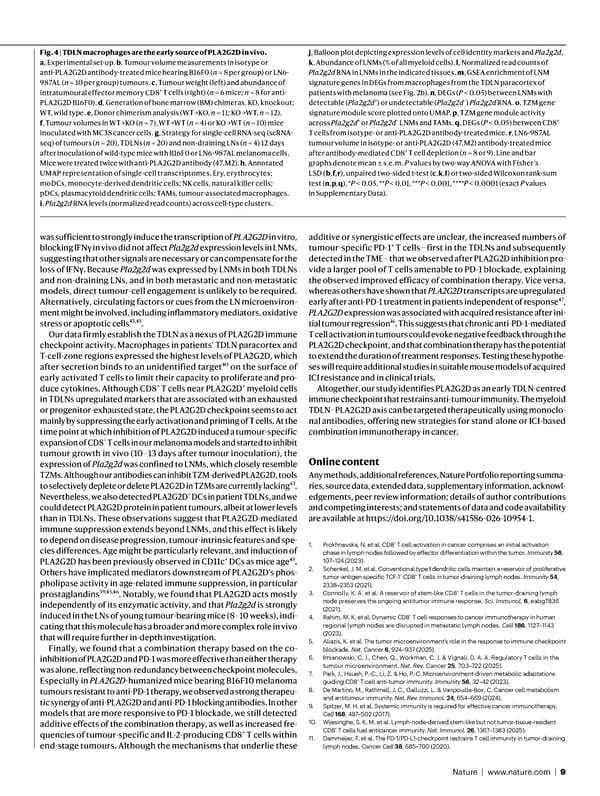
Nature | www.nature.com | 9 was sufficient to strongly induce the transcription of PLA2G2D in vitro, blocking IFNγ in vivo did not affect Pla2g2d expression levels in LNMs, suggesting that other signals are necessary or can compensate for the loss of IFNγ. Because Pla2g2d was expressed by LNMs in both TDLNs and non-draining LNs, and in both metastatic and non-metastatic models, direct tumour-cell engagement is unlikely to be required. Alternatively, circulating factors or cues from the LN microenviron- ment might be involved, including inflammatory mediators, oxidative stress or apoptotic cells 43,45 . Our data firmly establish the TDLN as a nexus of PLA2G2D immune checkpoint activity. Macrophages in patients’ TDLN paracortex and T-cell-zone regions expressed the highest levels of PLA2G2D, which after secretion binds to an unidentified target 40 on the surface of early activated T cells to limit their capacity to proliferate and pro- duce cytokines. Although CD8 + T cells near PLA2G2D + myeloid cells in TDLNs upregulated markers that are associated with an exhausted or progenitor-exhausted state, the PLA2G2D checkpoint seems to act mainly by suppressing the early activation and priming of T cells. At the time point at which inhibition of PLA2G2D induced a tumour-specific expansion of CD8 + T cells in our melanoma models and started to inhibit tumour growth in vivo (10–13 days after tumour inoculation), the expression of Pla2g2d was confined to LNMs, which closely resemble TZMs. Although our antibodies can inhibit TZM-derived PLA2G2D, tools to selectively deplete or delete PLA2G2D in TZMs are currently lacking 43 . Nevertheless, we also detected PLA2G2D + DCs in patient TDLNs, and we could detect PLA2G2D protein in patient tumours, albeit at lower levels than in TDLNs. These observations suggest that PLA2G2D-mediated immune suppression extends beyond LNMs, and this effect is likely to depend on disease progression, tumour-intrinsic features and spe - cies differences. Age might be particularly relevant, and induction of PLA2G2D has been previously observed in CD11c + DCs as mice age 45 . Others have implicated mediators downstream of PLA2G2D’s phos- pholipase activity in age-related immune suppression, in particular prostaglandins 39,45,46 . Notably, we found that PLA2G2D acts mostly independently of its enzymatic activity, and that Pla2g2d is strongly induced in the LNs of young tumour-bearing mice (8–10 weeks), indi- cating that this molecule has a broader and more complex role in vivo that will require further in-depth investigation. Finally, we found that a combination therapy based on the co- inhibition of PLA2G2D and PD-1 was more effective than either therapy was alone, reflecting non-redundancy between checkpoint molecules. Especially in PLA2G2D -humanized mice bearing B16F10 melanoma tumours resistant to anti-PD-1 therapy, we observed a strong therapeu- tic synergy of anti-PLA2G2D and anti-PD-1 blocking antibodies. In other models that are more responsive to PD-1 blockade, we still detected additive effects of the combination therapy, as well as increased fre- quencies of tumour-specific and IL-2-producing CD8 + T cells within end-stage tumours. Although the mechanisms that underlie these additive or synergistic effects are unclear, the increased numbers of tumour-specific PD-1 + T cells—first in the TDLNs and subsequently detected in the TME—that we observed after PLA2G2D inhibition pro- vide a larger pool of T cells amenable to PD-1 blockade, explaining the observed improved efficacy of combination therapy. Vice versa, whereas others have shown that PLA2G2D transcripts are upregulated early after anti-PD-1 treatment in patients independent of response 47 , PLA2G2D expression was associated with acquired resistance after ini- tial tumour regression 16 . This suggests that chronic anti-PD-1-mediated T cell activation in tumours could evoke negative feedback through the PLA2G2D checkpoint, and that combination therapy has the potential to extend the duration of treatment responses. Testing these hypothe- ses will require additional studies in suitable mouse models of acquired ICI resistance and in clinical trials. Altogether, our study identifies PLA2G2D as an early TDLN-centred immune checkpoint that restrains anti-tumour immunity. The myeloid TDLN–PLA2G2D axis can be targeted therapeutically using monoclo- nal antibodies, offering new strategies for stand-alone or ICI-based combination immunotherapy in cancer. Online content Any methods, additional references, Nature Portfolio reporting summa- ries, source data, extended data, supplementary information, acknowl- edgements, peer review information; details of author contributions and competing interests; and statements of data and code availability are available at https://doi.org/10.1038/s41586-026-10954-1. 1. Prokhnevska, N. et al. CD8 + T cell activation in cancer comprises an initial activation phase in lymph nodes followed by effector differentiation within the tumor. Immunity 56 , 107–124 (2023). 2. Schenkel, J. M. et al. Conventional type I dendritic cells maintain a reservoir of proliferative tumor-antigen specific TCF-1 + CD8 + T cells in tumor-draining lymph nodes. Immunity 54 , 2338–2353 (2021). 3. Connolly, K. A. et al. A reservoir of stem-like CD8 + T cells in the tumor-draining lymph node preserves the ongoing antitumor immune response. Sci. Immunol. 6 , eabg7836 (2021). 4. Rahim, M. K. et al. Dynamic CD8 + T cell responses to cancer immunotherapy in human regional lymph nodes are disrupted in metastatic lymph nodes. Cell 186 , 1127–1143 (2023). 5. Aliazis, K. et al. The tumor microenvironment’s role in the response to immune checkpoint blockade. Nat. Cancer 6 , 924–937 (2025). 6. Imianowski, C. J., Chen, Q., Workman, C. J. & Vignali, D. A. A. Regulatory T cells in the tumour microenvironment. Nat. Rev. Cancer 25 , 703–722 (2025). 7. Park, J., Hsueh, P.-C., Li, Z. & Ho, P.-C. Microenvironment-driven metabolic adaptations guiding CD8 + T-cell anti-tumor immunity. Immunity 56 , 32–42 (2023). 8. De Martino, M., Rathmell, J. C., Galluzzi, L. & Vanpouille-Box, C. Cancer cell metabolism and antitumour immunity. Nat. Rev. Immunol. 24 , 654–669 (2024). 9. Spitzer, M. H. et al. Systemic immunity is required for effective cancer immunotherapy. Cell 168 , 487–502 (2017). 10. Wijesinghe, S. K. M. et al. Lymph-node-derived stem-like but not tumor-tissue-resident CD8 + T cells fuel anticancer immunity. Nat. Immunol. 26 , 1367–1383 (2025). 11. Dammeijer, F. et al. The PD-1/PD-L1-checkpoint restrains T cell immunity in tumor-draining lymph nodes. Cancer Cell 38 , 685–700 (2020). Fig. 4 | TDLN macrophages are the early source of PLA2G2D in vivo. a , Experimental set-up. b , Tumour volume measurements in isotype or anti-PLA2G2D antibody-treated mice bearing B16F0 ( n = 8 per group) or LN6- 987AL ( n = 10 per group) tumours. c , Tumour weight (left) and abundance of intratumoural effector memory CD8 + T cells (right) ( n = 6 mice; n = 8 for anti- PLA2G2D B16F0). d , Generation of bone marrow (BM) chimeras. KO, knockout; WT, wild type. e , Donor chimerism analysis (WT→KO, n = 11; KO→WT, n = 12). f , Tumour volumes in WT→KO ( n = 7), WT→WT ( n = 4) or KO→WT ( n = 10) mice inoculated with MC38 cancer cells. g , Strategy for single-cell RNA-seq (scRNA- seq) of tumours ( n = 20), TDLNs ( n = 20) and non-draining LNs ( n = 4) 12 days after inoculation of wild-type mice with B16F0 or LN6-987AL melanoma cells. Mice were treated twice with anti-PLA2G2D antibody (47.M2). h , Annotated UMAP representation of single-cell transcriptomes. Ery, erythrocytes; moDCs, monocyte-derived dendritic cells; NK cells, natural killer cells; pDCs, plasmacytoid dendritic cells; TAMs, tumour-associated macrophages. i , Pla2g2d RNA levels (normalized read counts) across cell-type clusters. j , Balloon plot depicting expression levels of cell identity markers and Pla2g2d . k , Abundance of LNMs (% of all myeloid cells). l , Normalized read counts of Pla2g2d RNA in LNMs in the indicated tissues. m , GSEA enrichment of LNM signature genes in DEGs from macrophages from the TDLN paracortex of patients with melanoma (see Fig. 2b). n , DEGs ( P < 0.05) between LNMs with detectable ( Pla2g2d + ) or undetectable ( Pla2g2d − ) Pla2g2d RNA. o , TZM gene signature module score plotted onto UMAP. p , TZM gene module activity across Pla2g2d + or Pla2g2d − LNMs and TAMs. q , DEGs ( P < 0.05) between CD8 + T cells from isotype- or anti-PLA2G2D antibody-treated mice. r , LN6-987AL tumour volume in isotype- or anti-PLA2G2D (47.M2) antibody-treated mice after antibody-mediated CD8 + T cell depletion ( n = 8 or 9). Line and bar graphs denote mean ± s.e.m. P values by two-way ANOVA with Fisher’s LSD ( b , f , r ), unpaired two-sided t-test ( c , k , l ) or two-sided Wilcoxon rank-sum test ( n , p , q ). * P < 0.05, ** P < 0.01, *** P < 0.001, **** P < 0.0001 (exact P values in Supplementary Data).
 NATURE Paper - Published 9.9.26 - Apeximmune Page 8 Page 10